“At least I’m not a shrimp.”
It’s a line I’d often repeat to myself back in 2016, when I started taking animal suffering seriously and realized how fortunate I was to live a human life.
Of course, to most people this thought sounds entirely absurd, especially those who don’t take animal sentience seriously. But I figured if you accept that animals, like ourselves, are sentient, that each has an individual life, and that we only get to live one life on this planet, then the odds that I’d be born human, rather than as a shrimp (or some other animal whose life plan is basically “get eaten”), were astronomically small.
By some crude moral arithmetic, I estimated that for every one human born on this planet, somewhere between 70-700 trillion shrimp-like creatures were born, living short lives and meeting what I assumed were horrible deaths, likely being acidified inside a predator’s stomach.
I didn’t know whether this was fully accurate, but the possibility felt overwhelming. By sheer statistical luck, we won the jackpot of human existence, and did so in an era of unprecedented peace, medicine, knowledge, and wealth.
This shrimp sentience thought experiment is no longer just hypothetical. Whether shrimp can feel pain—and if so, how much—has become a central and increasingly serious debate within suffering-focused practical ethics, particularly among effective altruists (EAs), and has gained mainstream coverage in newspapers such as The Guardian [1] and Vox [2].
The 2021 report that set off EAs’ focus on this issue—Review of the Evidence of Sentience in Cephalopod Molluscs and Decapod Crustaceans [3]—was led by Jonathan Birch, who acted as the supervisor of my Master’s dissertation on how cognitive sophistication affects moral status. So as a former animal sentience student who is focused on reducing suffering, I felt compelled to dig into the evidence to see if my beliefs about moral priorities needed updating.
PART 1: SHRIMP
Why focus on shrimp
My default view has been that those who are serious about reducing suffering should focus on the plight of chickens. Not just because their living conditions are clearly bad [4,5], but precisely because they are so numerous [6], particularly when compared to cows [7], and the number we kill looks to keep growing rapidly for at least the next few decades [8,9]. I thus share most of the underlying beliefs of those who promote focus on shrimp welfare: the scale, tractability, and neglectedness of pain matter.
Shrimp are the perfect case to match this logic: their scale is enormous (farmed shrimp amount to close to half a trillion a year [10]—about five to six times as many as chickens, and more than 1,500 times as many as cows), their death seems painful (they tend to be killed in ice slurries, freezing to death [11]), improvements are highly tractable (simply using electric stunners rather than ice baths makes their death instant rather than potentially painful and drawn out), and, until recently, no one was doing anything about it.
The cost to improve things? About $1 per 1,000-1,500 shrimp that are switched from slowly freezing to being instantly electrically stunned to death [12]. May sound macabre, but if the logic holds, it’s hard to argue you can get a better welfare bang for your buck.
Despite their sheer number, I’ve historically placed less moral priority on aquatic animals like shrimp. Part of this is undoubtedly terrestrial bias, but much of it is evidential.
For wild-caught aquatic animals—the majority of seafood by biomass up until 2024 [13]—I’ve never been too convinced that human capture is that morally distinctive from the violent deaths these animals would otherwise face in nature. Among farmed ones, the welfare picture is also far less clear than it is for terrestrial livestock [14]: we lack strong evidence that their lives are dominated by the kinds of chronic growth disorders, infections, and injuries that seem to make the lives of animals like chickens a net negative [15,16].
Most importantly, we simply weren’t sure whether many aquatic animals feel pain at all [14]. While the evidence for pain in fish has grown increasingly persuasive [3], shrimp in particular remained a genuine question mark.
Enter Birch’s work. In his 2024 book The Edge of Sentience [17], he offers a framework for decision-making under uncertainty about a being’s sentience. He argues that when there is credible evidence placing one near the “edge of sentience,” the asymmetry of moral risk favors precaution: the harm of mistakenly denying sentience to a sentient being is typically much greater than the harm of mistakenly extending protections to a non-sentient one.
His sentience framework reviews evidence for sentience across eight criteria:
1. Presence of nociceptors
2. Integrative brain regions
3. Connections between nociceptors and integrative brain regions
4. Responses affected by local anesthetics or analgesics
5. Motivational trade-offs
6. Flexible self-protective behavior
7. Associative learning that goes beyond habituation or sensitization
8. Behavior indicating valuation of analgesia
As more of these criteria are met, Birch argues, it becomes increasingly implausible that no phenomenological, subjectively felt experience is present. At some point, it is more reasonable to assume that the animal feels something, however minimal, than that it performs complex behavior in a complete experiential vacuum [17].
His decapod review, which recommends “that all cephalopod molluscs and decapod crustaceans be regarded as sentient animals for the purposes of UK animal welfare law,” [3] (p.8) has been highly influential. It helped inform the UK government’s decision to include crustaceans within animal welfare law [18,19]—effectively banning practices such as boiling lobsters alive—and now serves as the central evidence cited by shrimp welfare advocates.
The evidence for shrimp pain
What should stand out right away in the decapod review is that the evidence varies dramatically across taxa. Among the six decapod taxa reviewed, true and anomuran crabs have been relatively well-studied, astacid lobsters, spiny lobsters, and caridean shrimp less so, and the shrimp species most commonly consumed by humans—Litopenaeus vannamei [20,21]; part of the penaeid shrimp family and the focus of shrimp welfare projects—sits at the bottom of this evidence spectrum.
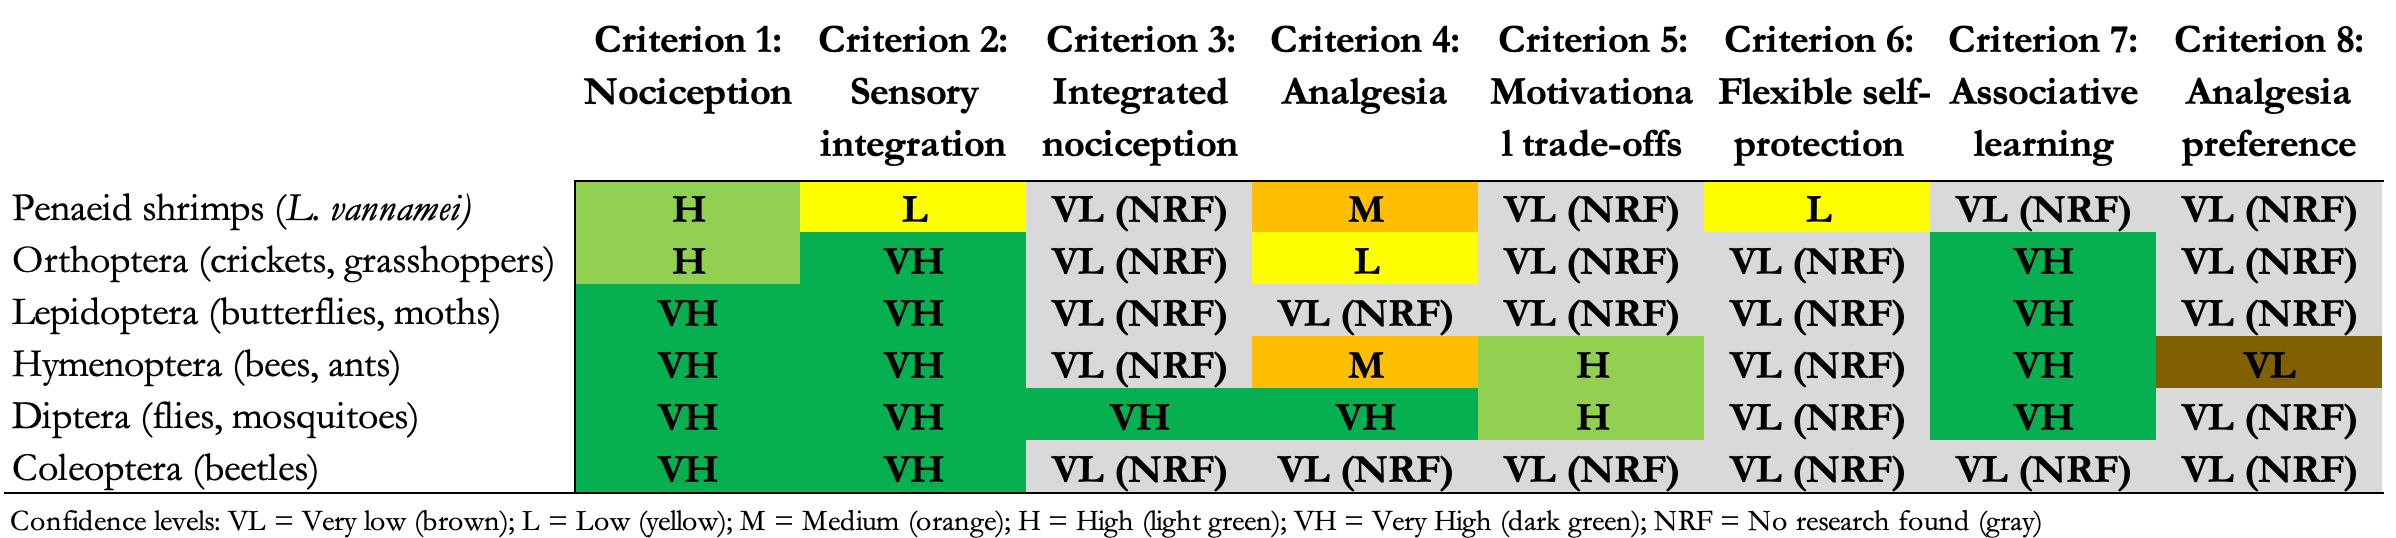
L. vannamei scores low confidence on all but two of the eight criteria, the exceptions being (1) presence of nociceptors and (4) responses affected by local anesthetics or analgesics. Importantly, “low confidence” for a criterion here often means we don’t know, rather than negative findings: absence of evidence is not evidence of absence, and L. vannamei remains understudied on most of the criteria [3] (p.6).
The most direct behavioral finding supporting pain experience in L. vannamei is that during the common industry procedure of eyestalk ablation—the cutting of one or both eyestalks to accelerate maturation [22,23]—they exhibit reactions such as erratic swimming and tail flicking, which is reduced by the topical application of the anesthetic lidocaine [24].
This suggests the reaction may involve nociceptive pathways that can be dampened pharmacologically, which is consistent with possible pain experience. But rather than specific relief of pain or an aversive state, it could also simply reflect generalized motor suppression or reduced responsiveness.
Beyond this, the picture for L. vannamei is muddy. One study on a caridean shrimp species—not peneaid, like L. vannamei—called Palaemon elegans, found that exposure of one antenna to low-pH acetic acid or high-pH sodium hydroxide elicited location-specific grooming and rubbing behavior—indicative of pain or irritation—which was attenuated by the local anesthetic benzocaine [25].
However, a later study, using three decapods—including the penaeid shrimp Litopenaeus setiferus, a close relative of L. vannamei—found no such directed grooming or rubbing, even when stronger pH stimuli were used [26].
Given the lack of solid direct evidence, the case for pain in L. vannamei is thus often an argument by association: better-studied decapods such as crabs and lobsters show evidence of pain-like behavior, so it’s argued that L. vannamei likely has similar capacities [27].
As noted, the decapod report concludes with the recommendation to include all decapods, including L. vannamei, in animal welfare law. But Birch is candid about what this policy recommendation actually rests on.
In the conclusion, he writes:
“We have noted that there is very little evidence of sentience at present in penaeid [including L. vannamei] shrimps. However, if caridean shrimps were included, but penaeid [L. vannamei] shrimps excluded, the potential for confusion [emphasis added] would be high. Therefore, on balance, we reject the suggestion that protection should only be extended to specific infraorders of decapod.” [3] (p.81)
L. vannamei gets included not because the evidence converges on “sentience looks likely,” but because excluding them while including other shrimps would make the law confusing in practice. So even within Birch’s broadly precautionary posture, L. vannamei are an awkward outlier, included for administrative clarity rather than scientific confidence.
Three years after the decapod report, he sharpens and explains this choice in his book [17], noting that a neuroanatomical survey found that decapods generally have “hemiellipsoid bodies” [28]—integrative regions linked to learning and memory—but that in L. vannamei specifically, these regions appear miniaturized and weakly differentiated [17] (p.256).
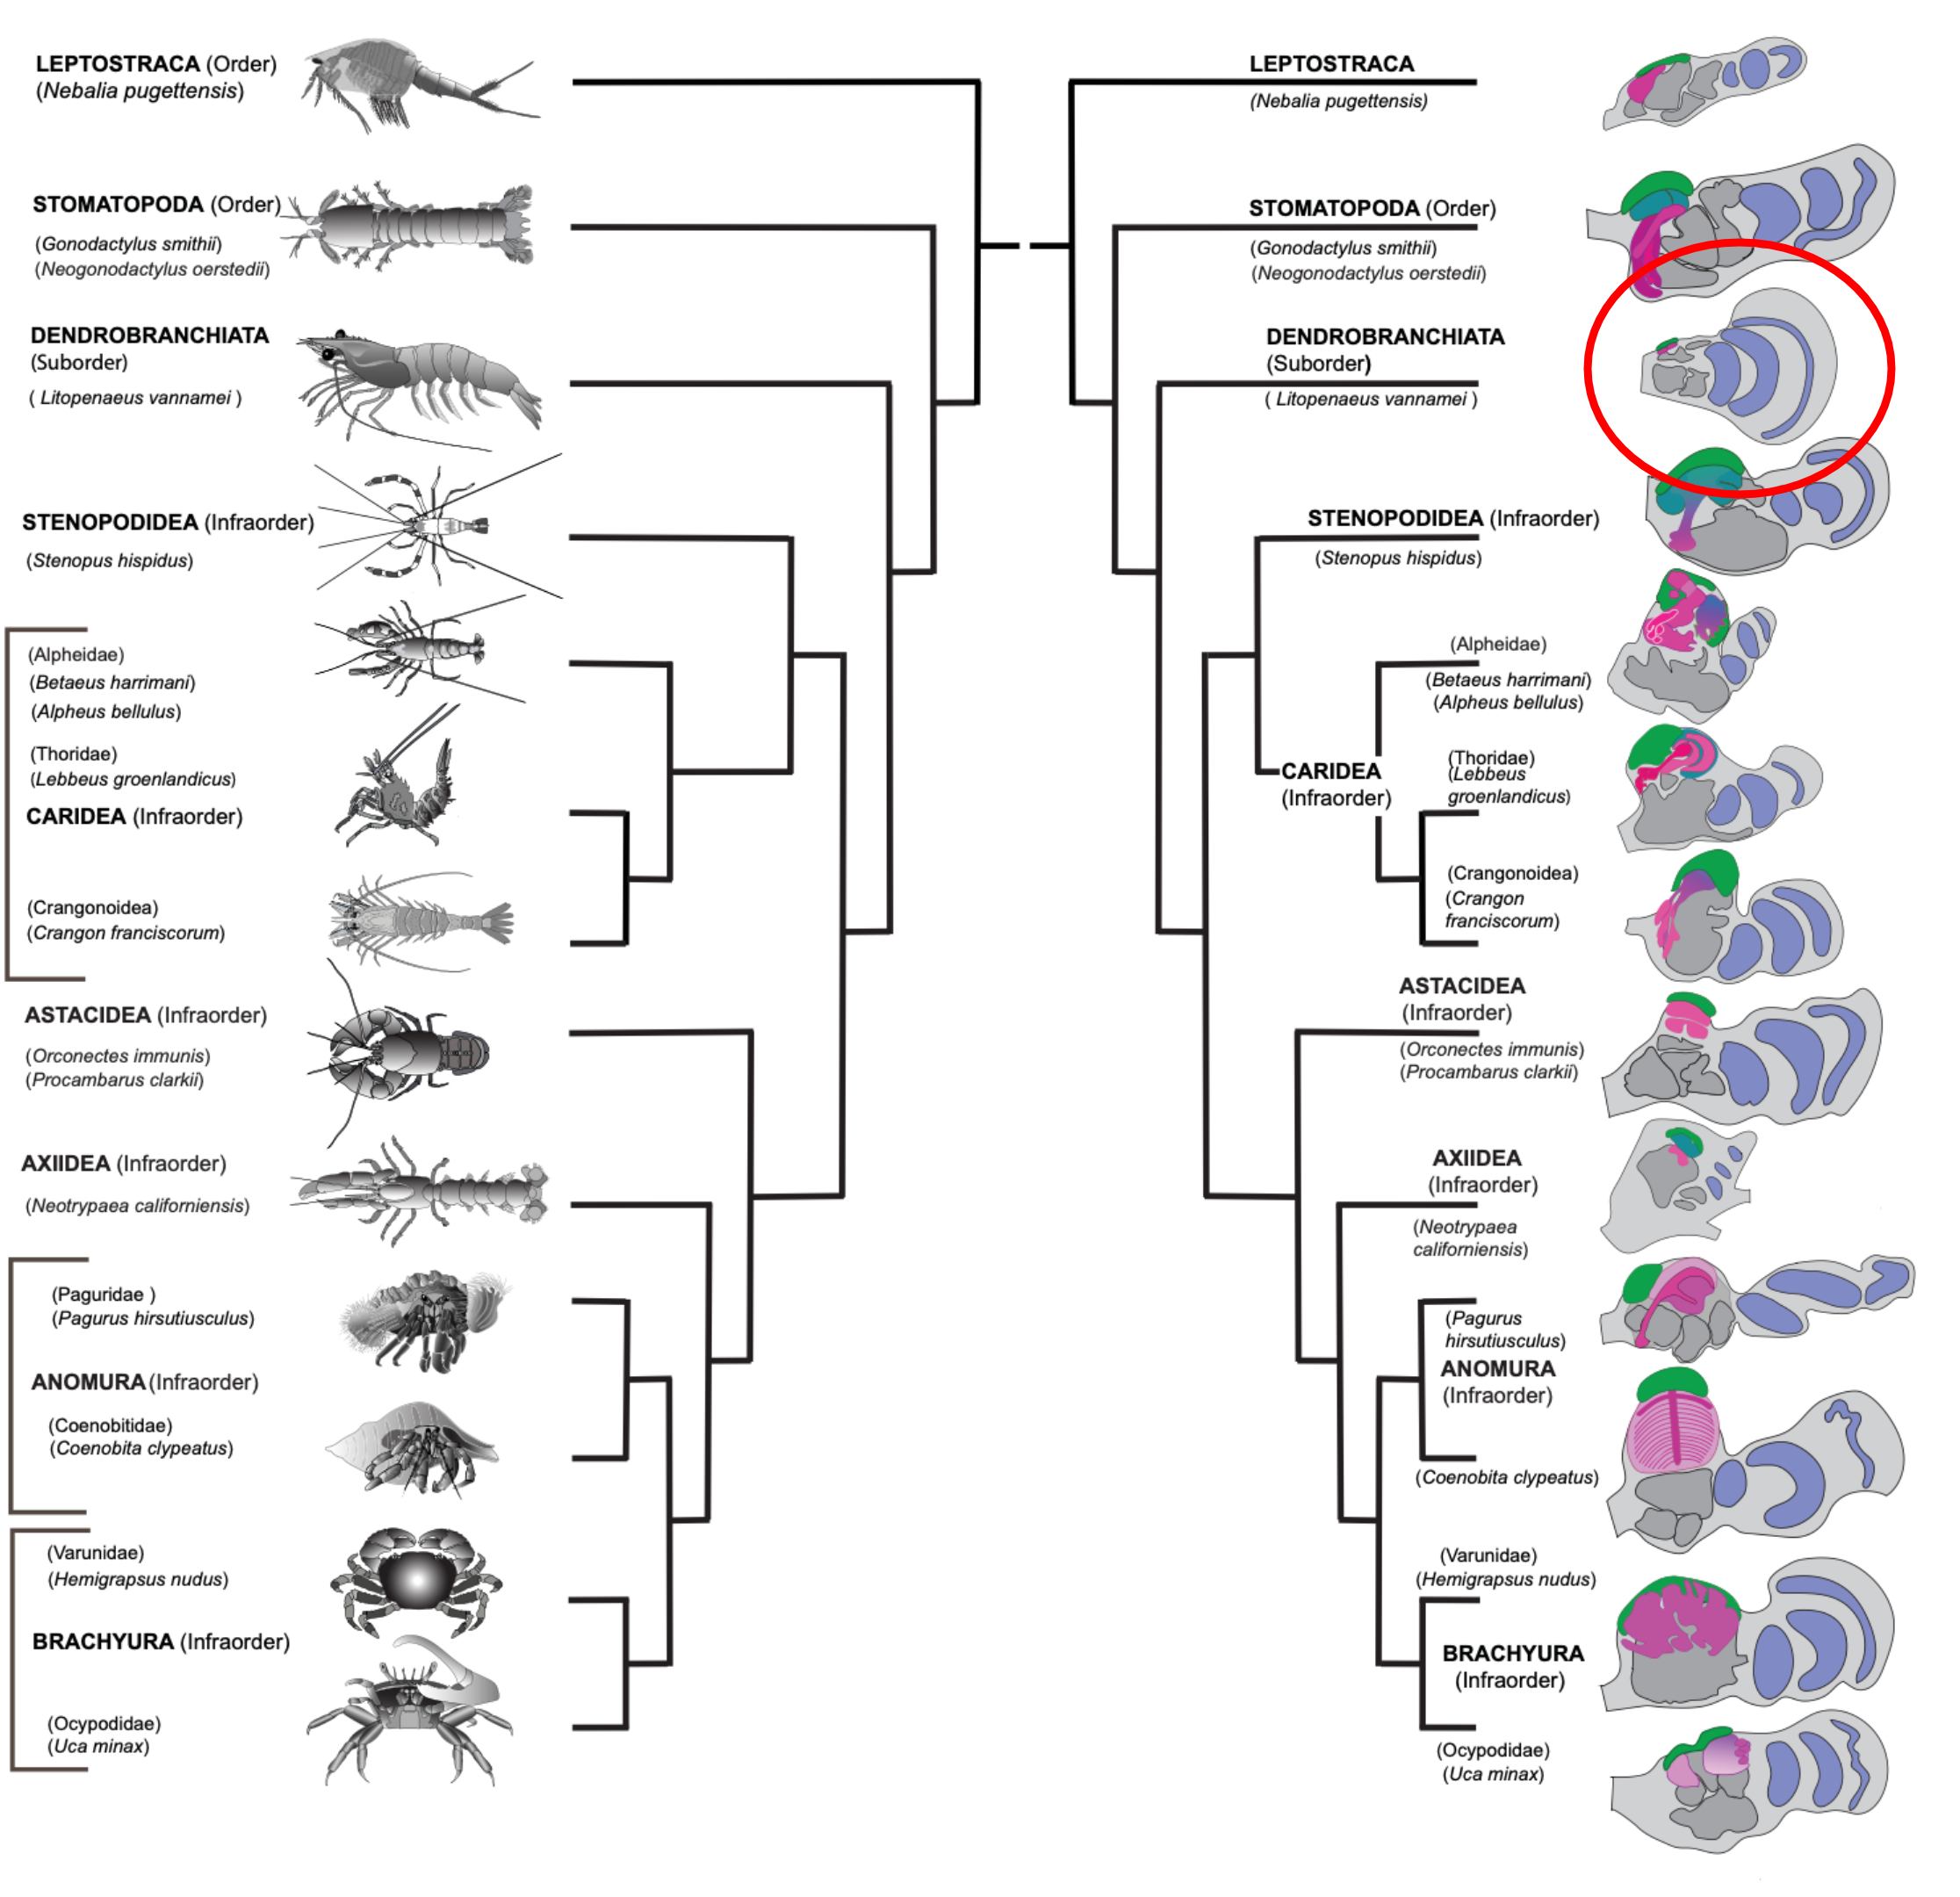
Birch emphasizes why this matters: nervous tissue is metabolically expensive to run, so dramatic reduction is often what we expect to see when a system is no longer functionally significant. On this basis, he reports low confidence that L. vannamei has functional integrative brain regions—not that such regions are entirely absent, but that they may not do substantial integrative work. Without integration, it becomes harder to confidently argue an animal is feeling pain, rather than merely reacting through nociceptors.
He then draws a sharper taxonomic line: Pleocyemata—walking decapods and caridean shrimps—do count as sentience candidates (the evidence is substantial enough to warrant some precaution), while Dendrobranchiata, which include penaeid shrimps such as L. vannamei, do not [17] (p.258-262). In other words, across the six decapods he reviews, L. vannamei is the only one he does not class as a sentience candidate.
And that matters, because the move made by some shrimp advocates is extrapolation: if crabs and lobsters show pain-like responses, it is argued shrimp probably do too. For example, one commonly cited welfare-range model explicitly approximates shrimp’s probability of sentience as equivalent to the prior distribution used for crabs [29]. But critics point out that, given the structural differences between decapod lineages, this kind of taxonomic borrowing across suborders is shaky [30].
None of this is a full denial of sentience in L. vannamei, and Birch entertains the possibility that some lineages could evolve integrative capacities and later lose them. But the practical conclusion he draws is that L. vannamei is precisely a case where the integrative-architecture story looks too insecure and the evidential base too thin to treat sentience as likely, even within a precautionary framework [17] (p.257-258).
Because of the lack of research on L. vannamei and potentially large welfare stakes, Birch places them into the “investigative priority” category, together with beings such as worms and insect larvae [17] (p.276-281).
Skepticism
The overall L. vannamei evidence picture, in terms of where (very few) studies actually exist, thus looks roughly like this: there is high confidence that they (1) possess nociceptors and medium confidence that (4) their responses can be modulated by local anesthetics or analgesics [3,24]. There is low confidence that they (2) have functional integrative brain regions [3,28] or (6) that they show self-protective behavior in response to noxious stimulation [3,26].
There appear to be no studies bearing on (3) connections between nociceptors and integrative brain regions, (5) motivational trade-offs, (7) associative learning, or (8) behavior suggesting valuation of analgesia. And while that absence is not decisive, it matters that in practice, when we have strong evidence for the higher-order criteria (5–8), it usually comes from systems where we also have at least some independent support for integrative circuitry (2).
Even allowing for selection effects, nociceptors and pharmacological modulation are doing virtually all the work here—features that are widespread and not strongly diagnostic on their own. And if we can’t safely generalize from related taxa, the sentience case for L. vannamei becomes extremely thin.
A plausible reason we commonly see framing along the lines of “we just haven’t studied shrimp enough yet, but it’s reasonable to assume they likely feel pain based on other decapods” is Birch et al.’s confidence scoring itself. In their system, low confidence can reflect two very different situations: either that a criterion has not been investigated in the relevant species, or that it has been investigated and the results have been weak or negative.
As a result, it is easy to read the gap between shrimp and better-studied decapods as only a research gap. And to a large extent, that’s true. But the limited evidence that is available is unsupportive on two important pain-relevant markers. This ambiguity in what “low confidence” denotes—an issue brought up by critics of Birch’s original approach [30], which he appears to have addressed in later reports [31]—could therefore blur the distinction between “we don’t know yet” and “the evidence so far leans against”.
Another place where some caution about confidence is warranted is the welfare impact of ice slurry, the slaughter method often contrasted with electrical stunning.
Electrical stunning is rightly treated as one of the most humane commercially available options because it is designed to render animals rapidly insensible [33]. However, Birch, while recommending it as best current practice based on the available evidence (and indeed ahead of ice slurry), is explicit that we still don’t know what the neural activity induced by electrical stunning feels like from the animal’s point of view, or whether the resulting unresponsive state is truly unconsciousness rather than some form of continuing experience [3] (p.71-72).
At the same time, we also don’t fully know whether chilling (from ice slurry) is actually painful in shrimp [3] (p.73) [34], and its effects are at least not uniform across species. One review notes that lobsters and crabs retained sensory-central nervous system responses in very cold conditions—suggesting chilling may not reliably anesthetize them—but for L. vannamei it describes a rapid collapse in activity when transferred to ice, interpreted by the authors as consistent with anesthesia [33]. This is a liberal interpretation, however, since reduced activity alone cannot establish insensibility.
None of this shows that ice slurry is humane or painless, and electrical stunning does have the strongest welfare-based rationale. But it does make confident “ice = obvious agony” or “electrical stunning = painless” harder to state as if it’s fact. The Shrimp Welfare Project is trying to get more peer-reviewed scientific data on this issue [11], which is a good thing.
This is also not at all to say that the science on L. vannamei is anywhere near settled, or that more evidence on their potential sentience isn’t needed. But I do think taking the case seriously based on current evidence opens an—almost literally—enormous can of worms.
PART 2: PRIORITIZATION
The implications of this view
Indeed, if one does consider the case for L. vannamei as being enough to warrant precaution and acting on it, then Birch’s own consistency arguments make it hard to deny comparable consideration to at least ants, fruit flies, and mosquitoes.
In fact, when these same sentience criteria are applied to insects, as Birch and colleagues have done in another report, flies and mosquitoes score high to very high confidence evidence for six out of eight criteria, and ants do so for four out of eight, compared to only one criterion for L. vannamei [31]. Importantly, this includes a functional central complex that L. vannamei appears to lack. Birch indeed proposes that, unlike L. vannamei, all adult insects are sentience candidates [17] (p.272).
We currently farm and kill about one trillion insects, and this is expected to increase to about ten trillion by 2030 [34] (though estimates vary). Slaughter methods include boiling, freezing, freeze-drying, blast drying, spraying with hot water, mechanical crushing, and shredding [17] (p.294), most if not all of which may be extremely painful.
By precautionary expected value reasoning, insects appear to make a stronger case than shrimp: they show more markers of sentience, are much larger in (projected) scale, and killed in equally (if not more) seemingly painful ways. Tractability might be one point where shrimp is stronger, though active work on insect welfare practices [35], instantaneous killing [35,36], and humane insecticides [37] could well exceed it there too.
Birch’s framework is designed for ethical decision-making under uncertainty, where the evidence is incomplete, and the potential downside of getting it wrong could be massive. The difficulty is that, once you combine this precautionary posture with EA-style expected value reasoning, the moral priorities landscape easily gets hijacked by these low-probability, ultra-high-scale cases.
Insects are stitched into the basic metabolism of life: conservative estimates place annual insect deaths in agriculture at hundreds of trillions; others, once you include pesticides, habitat destruction, and crop harvesting, estimate around 3.5 quadrillion [17,37]. That’s about half a million insects per human per year.
A tiny credence multiplied by an astronomical number of individuals multiplied by even very modest negative experience thus threatens to dominate moral attention. If one considers shrimp welfare as the “precautionary frontier,” by this logic, insects aren’t at the frontier, but already over the line. On this view, the main ethical crisis built into modern life is the quadrillions of insects we kill just to move around, wash, and eat food—under our shoes, beneath our tires, in our sinks, and across our food crops.
And there the epistemic problem becomes practical: when you cut back on meat, you can tell a legible story—avoid something like ~10 chicken meals and, roughly, one chicken doesn’t have to be raised and killed—but with insects you can’t even define, let alone verify, the “insects not killed” counterfactual, so the moral arithmetic starts to outrun anything a human can responsibly act on. Just one fruit salad might rack up more deaths than your conscience can even render.
We can accept this “moral explosion” if we think it is simply the logical consequence of an otherwise coherent worldview—one that gestures toward something Benatarian: a view on which the cleanest way to reduce suffering appears to be to reduce sentient life itself [38]. That’s not to say it’s definitively wrong; perhaps the world really is largely made up of enormous invertebrate suffering.
Alternatively, we can try to add principled constraints that prevent low-confidence, ultra-high-n cases from hijacking the moral landscape.
Birch manages some of the high-n runaway logic through proportionality (distinguishing unavoidable collateral harms from avoidable, high-risk practices; e.g., accidentally stepping on an ant vs. killing ants for food without effective stunning) [17] (p.154-170); democratic deliberation (using informed citizen processes to settle what trade-offs are proportionate) [17] (p.138-153); and making distinctions between sentience candidates and investigation priorities (the former getting precaution, the latter urgently needing more research) [17] (p.123-127), which are sensible brakes for governance as they prevent policy whiplash.
However, besides it seeming unlikely people will ever care about mosquito welfare—even after fifty years of modern animal advocacy [39] there is little evidence of a shift away from industrially farmed animal products at the population level, with chicken slaughter per person roughly quadrupling during this period [6,7]—these constraints don’t solve the cause-prioritization problem, because they don’t tell you how to compare 10 billion high-confidence extreme sufferers against 10 trillion low-confidence ones.
And even granting the usual EA filters—tractability, neglectedness, feasibility, and evidential robustness—the scale gradient from shrimp to insects (via agriculture-related deaths) is so steep that these filters don’t, by themselves, explain why the precautionary logic should settle on shrimp. All else equal, once you shift to a target that is thousands of times larger, an intervention could be far less effective and still compete on expected impact.
Pain severity
I think it helps here to consider a few observations that Birch collects that sit awkwardly with our usual inferences about severe suffering.
He notes that insects “will continue normal feeding and mating behaviours despite catastrophic injury” [17] (p.264), with examples including “a dragonfly eating its own detached abdomen” and “a sleeping moth that is not woken by being pinned to a tree” [17,40] (p.264).
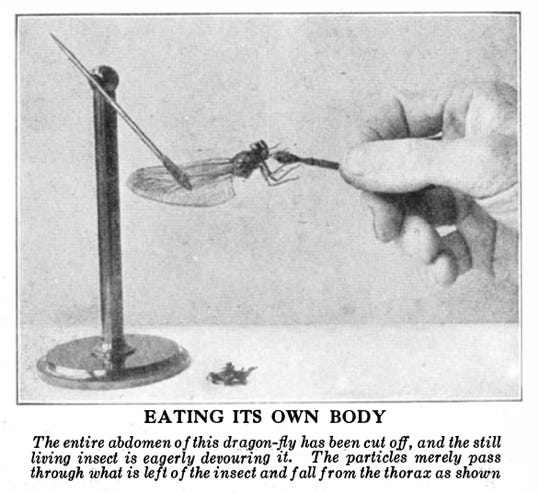
Though based on observation rather than experimentation, Eisemann et al. provide a vivid illustration of the pain severity-inference problem in insects:
“… our experience has been that insects will continue with normal activities even after severe injury or removal of body parts. An insect walking with a crushed tarsus, for example, will continue applying to the substrate with undiminished force. Among our other observations are those on a locust which continued to feed whilst itself being eaten by a mantis; aphids continuing to feed whilst being eaten by coccinellids; a tsetse fly which flew in to feed although half-dissected; caterpillars which continue to feed whilst tachinid larvae bore into them; many insects which go about their normal life whilst being eaten by large internal parasitoids; and male mantids which continue to mate as they are being eaten by their partners.” [41]
Recent work has argued that these observations are easy to misinterpret. “Normal” post-injury behavior may be confounded by insect-specific biomechanics, such that injury in insects may look different. When insects’ gaits are measured, for example, changes have been observed in how they walk post-injury. It’s also plausible that a sense of threat may have suppressed their injury responses in these cases, and that the vivid examples described are atypical [42]. Further, there is evidence consistent with self-protection and valuation in some insects, such as wound-tending in cockroaches and moth larvae [31], and motivational trade-offs in fruit flies [43] and bees [31,44].
Yet it is possible that a system can implement aversion and learning without supporting integrated, life-dominating negative states. This remains a substantive assumption, and one that we may never get definitive answers to. Indeed, the current insect and broader sentience literature is better at answering “can they respond to noxious stimuli?” than “can they enter states of severe and disabling distress?” Sentience markers often function as threshold tests, but they’re poorly calibrated to severity.
The issue with severity is that it’s a felt state that we don’t get access to in other species—in humans, severity is mainly inferred from self-report. However, if catastrophic injury does leave basic feeding and mating behavior broadly intact in a system, then plausible interpretations are that the system only supports highly local, easily overridden aversion, that it can compartmentalize to an extreme extent, or that it has no felt aversive experience at all. I also think it’s worth asking here what observable patterns can count as evidence against a system being capable of experiencing severe life-dominating distress to prevent “severity” from becoming insulated from evidence; spectacular tolerance to ripped off limbs, if commonly observed, would certainly count against it.
In terms of moral priority setting, severity weighting seems attractive, which can be encoded as a strict override (the controversial lexical priority view that even a moment of excruciating pain defeats any amount of moderate discomfort, which has serious issues [45]), or more modestly as extreme weights that make “disabling” or “excruciating” pain dominate “annoying” or “hurtful” pain by large orders of magnitude.
There is some empirical support for this: when people evaluate aversive episodes, they tend to strongly weight peak intensity and are largely insensitive to duration [46–52], while ratings of pain unpleasantness increase extremely nonlinearly with intensity [53–55]. The Welfare Footprint Institute’s categories make this discontinuity in pain explicit: “annoying” and “hurtful” still leave room for positive welfare, whereas “disabling” and “excruciating” are, by definition, inconsistent with it [53].
While a large number of local aversions still matter on this view, what should dominate moral attention are the kinds of aversive states that crowd out any possibility of positive experience. The critical question, of course, is whether shrimp or insects can experience these states.
Prioritization
Shrimp welfare combines several features that make an intervention attractive. It covers very large numbers, can be implemented clearly, and may result in large welfare gains at low cost. On a precautionary view, it appears like a reasonable place to act, and it may create industry spillovers for other aquatic invertebrates as well—simply stunning animals before killing them is a pretty low bar.
But the case is weaker than how advocates often portray it, because the flagship species, L. vannamei, is supported by extremely thin evidence. Beyond nociceptors and pharmacological modulation, there is no good evidence for sentience. Among the six decapods Birch has reviewed, it is telling that he only excludes L. vannamei from sentience candidacy. Decisively responding to that level of uncertainty logically extends to insects more strongly, given their stronger sentience markers and their vastly larger numbers. (And they are, indeed, considered “sentience candidates”.)
Some of the friction is practical as well. Shrimp welfare is (for now), unavoidably, a bet. If they turn out not to be sentient, which I think is plausible given current evidence, the direct welfare impact of intervening collapses to near zero (leaving only the aforementioned spillovers like better industry standards). That’s a different kind of pay-off than investing in interventions for high-certainty-sentience beings.
I think a portfolio view with heavy emphasis on proven, serious suffering makes sense here, with the bulk of resources going into high-confidence disabling to severe suffering, especially if there are proven interventions, and a smaller share going to high-n uncertain cases. Shrimp welfare would become a lot more compelling to me if confidence accumulates for a basic sentience criterion outside of nociception—especially a higher-order one (5-8).
Disclosure: I’m not neutral. I’ve focused on chicken welfare since at least 2017. I should also note that in my 2020 LSE thesis I defended a fairly binary view of pain—either a being can suffer in a robust way, or it can’t suffer at all—I’m less confident in that picture now. Some of that is genuine updating, but some of it might be motivated reasoning too.
Update: Feb 6, 2026 — changed some wording based on some thoughts from Bob Fischer on the article.
References
1. Stock P. Do prawns feel pain? Why scientists are urging a rethink of Australia’s favoured festive food. The Guardian [Internet]. 2025 Dec 21 [cited 2026 Jan 8]; Available from: https://www.theguardian.com/world/2025/dec/22/crustaceans-feelings-sentient-christmas-new-year-prawns-australia
2. Matthews D. The case for caring about shrimp. Vox [Internet]. 2025 Sep 11 [cited 2026 Jan 8]; Available from: https://www.vox.com/future-perfect/461008/shrimp-welfare-project-controversy
3. Birch J, Burn C, Schnell A, Browning H, Crump A. Review of the Evidence of Sentience in Cephalopod Molluscs and Decapod Crustaceans [Internet]. London School of Economics and Political Science; 2021 Jan. Available from: https://www.lse.ac.uk/News/News-Assets/PDFs/2021/Sentience-in-Cephalopod-Molluscs-and-Decapod-Crustaceans-Final-Report-November-2021.pdf.
4. Schuck-Paim C, Alonso WJ. Quantifying Pain in Broiler Chickens: Impact of the Better Chicken Commitment and Adoption of Slower-Growing Breeds on Broiler Welfare. 2022. 458 p.
5. Schuck-Paim C, Alonso WJ. Quantifying Pain in Laying Hens: A blueprint for the comparative analysis of welfare in animals. 2021. 338 p.
6. Surveys - Poultry Slaughter [Internet]. United States Department of Agriculture - National Agricultural Statistics Service; 2024. Available from: https://www.nass.usda.gov/Surveys/Guide_to_NASS_Surveys/Poultry_Slaughter/index.php
7. Surveys - Livestock Slaughter [Internet]. United States Department of Agriculture - National Agricultural Statistics Service; 2024. Available from: https://www.nass.usda.gov/Surveys/Guide_to_NASS_Surveys/Livestock_Slaughter/index.php
8. Global meat consumption [Internet]. Our World in Data. [cited 2026 Jan 20]. Available from: https://ourworldindata.org/grapher/global-meat-projections-to-2050
9. Jia J, Dawson TP, Wu F, Han Q, Cui X. Global meat demand projection: Quo Vadimus? Journal of Cleaner Production. 2023 Dec 1;429:139460.
10. McKay H. Three Numbers That Make The Case For Shrimp Welfare [Internet]. Faunalytics. 2024 [cited 2026 Jan 20]. Available from: https://faunalytics.org/three-numbers-that-make-the-case-for-shrimp-welfare/
11. Humane Slaughter for Shrimp: Q&A with Shrimp Welfare Project [Internet]. Shrimp Insights. 2026 [cited 2026 Jan 20]. Available from: https://www.shrimpinsights.com/advertorial/humane-slaughter-shrimp-qa-shrimp-welfare-project
12. (Shr)Impact [Internet]. Shrimp Welfare Project. [cited 2026 Jan 11]. Available from: https://www.shrimpwelfareproject.org/shrimpact
13. The State of World Fisheries and Aquaculture [Internet]. Food and Agriculture Organization of the United Nations; 2024 [cited 2026 Jan 11]. Available from: https://www.fao.org/publications/fao-flagship-publications/the-state-of-world-fisheries-and-aquaculture/en
14. Browman HI, Cooke SJ, Cowx IG, Derbyshire SWG, Kasumyan A, Key B, et al. Welfare of aquatic animals: where things are, where they are going, and what it means for research, aquaculture, recreational angling, and commercial fishing. ICES J Mar Sci. 2019 Jan 1;76(1):82–92.
15. Bessei W. Welfare of broilers: a review. World’s Poultry Science Journal. 2006 Sep;62(3):455–66.
16. Broilers | Pain Track [Internet]. Welfare Footprint Institute. [cited 2026 Jan 11]. Available from: https://cp.pain-track.org/broilers
17. Birch J. The Edge of Sentience: Risk and Precaution in Humans, Other Animals, and AI [Internet]. Oxford University Press; 2024 [cited 2026 Jan 11]. Available from: https://doi.org/10.1093/9780191966729.001.0001
18. Lobsters, octopus and crabs recognised as sentient beings [Internet]. GOV.UK. [cited 2026 Jan 11]. Available from: https://www.gov.uk/government/news/lobsters-octopus-and-crabs-recognised-as-sentient-beings
19. Courea E. Boiling lobsters alive to be banned in England amid animal cruelty crackdown. The Guardian [Internet]. 2025 Dec 22 [cited 2026 Jan 11]; Available from: https://www.theguardian.com/world/2025/dec/22/boiling-lobsters-alive-banned-animal-cruelty-crackdown
20. Liao IC, Chien YH. The Pacific White Shrimp, Litopenaeus vannamei, in Asia: The World’s Most Widely Cultured Alien Crustacean. In: Galil BS, Clark PF, Carlton JT, editors. In the Wrong Place - Alien Marine Crustaceans: Distribution, Biology and Impacts [Internet]. Dordrecht: Springer Netherlands; 2011 [cited 2026 Jan 11]. p. 489–519. Available from: https://doi.org/10.1007/978-94-007-0591-3_17
21. Cheney J. An Overview of Shrimp and its Sustainability in 2024 [Internet]. 2024 [cited 2026 Jan 11]. Available from: https://sustainablefisheries-uw.org/shrimp-sustainability-2024/
22. Lumare F. Reproduction of Penaeus kerathurus using eyestalk ablation. Aquaculture. 1979 Nov 1;18(3):203–14.
23. Sainz-Hernández JC, Racotta IS, Dumas S, Hernández-López J. Effect of unilateral and bilateral eyestalk ablation in Litopenaeus vannamei male and female on several metabolic and immunologic variables. Aquaculture. 2008 Oct 1;283(1):188–93.
24. Taylor J, Vinatea L, Ozorio R, Schuweitzer R, Andreatta ER. Minimizing the effects of stress during eyestalk ablation of Litopenaeus vannamei females with topical anesthetic and a coagulating agent. Aquaculture. 2004 Apr 26;233(1):173–9.
25. Barr S, Laming PR, Dick JTA, Elwood RW. Nociception or pain in a decapod crustacean? Animal Behaviour. 2008 Mar 1;75(3):745–51.
26. Puri S, Faulkes Z. Do Decapod Crustaceans Have Nociceptors for Extreme pH? PLOS ONE. 2010 Apr 20;5(4):e10244.
27. Are Shrimps Sentient? [Internet]. Shrimp Welfare Project. [cited 2026 Jan 12]. Available from: https://www.shrimpwelfareproject.org/are-shrimps-sentient
28. Strausfeld NJ, Wolff GH, Sayre ME. Mushroom body evolution demonstrates homology and divergence across Pancrustacea. Behrens TE, Carr CE, Carr CE, Osorio D, Katz P, editors. eLife. 2020 Mar 3;9:e52411.
29. Fischer. Rethink Priorities’ Welfare Range Estimates [Internet]. Rethink Priorities. 2023 [cited 2026 Jan 26]. Available from: https://rethinkpriorities.org/research-area/welfare-range-estimates/
30. Mallatt J, Feinberg TE. Decapod sentience: Promising framework and evidence. Animal Sentience. 2022 Jan 1;7:1.
31. Gibbons M, Crump A, Barrett M, Sarlak S, Birch J, Chittka L. Can insects feel pain? A review of the neural and behavioural evidence. In: Advances in Insect Physiology [Internet]. Academic Press; 2022 [cited 2026 Jan 12]. p. 155–229. Available from: https://www.sciencedirect.com/science/chapter/bookseries/pii/S0065280622000170
32. Rotllant G, Llonch P, García del Arco JA, Chic Ò, Flecknell P, Sneddon LU. Methods to Induce Analgesia and Anesthesia in Crustaceans: A Supportive Decision Tool. Biology. 2023 Mar;12(3):387.
33. McKay H, McAuliffe W, Romero Waldhorn D. Welfare considerations for farmed shrimp. 2023 Dec 7 [cited 2026 Jan 22]; Available from: https://osf.io/yafqv
34. Barrett M, Fischer B. Challenges in farmed insect welfare: Beyond the question of sentience. Anim Welf. 2023 Jan 26;32:e4.
35. Insects raised for food and feed — global scale, practices, and policy [Internet]. Rethink Priorities. 2020 [cited 2026 Jan 23]. Available from: https://rethinkpriorities.org/research-area/insects-raised-for-food-and-feed/
36. Barrett M, Miranda C, Veloso IT, Flint C, Perl CD, Martinez A, et al. Grinding as a slaughter method for farmed black soldier fly (Hermetia illucens) larvae: Empirical recommendations to achieve instantaneous killing. Anim Welf. 2024 Mar 12;33:e16.
37. Howe H. Improving pest management for wild insect welfare [Internet]. Wild Animal Initiative. 2021 [cited 2026 Jan 23]. Available from: https://www.wildanimalinitiative.org/library/humane-insecticides
38. Benatar D. The Human Predicament: A Candid Guide to Life’s Biggest Questions. New York: Oxford University Press; 2017. 288 p.
39. Singer P, Harari YN. Animal Liberation Now: The Definitive Classic Renewed. New York: Harper Perennial; 2023. 368 p.
40. Bastin H. Do Insects Feel Pain? Scientific American. 1927;137(6):531–531.
41. Eisemann C, Jorgensen W, Rice M, Cribb B, Webb P, Zalucki M. Do insects feel pain? — A biological view. Experientia. 1984 Feb 1;40:164–7.
42. Barrett M, Fischer B. The Era beyond Eisemann et al. (1984): Insect Pain in the 21st Century. The Quarterly Review of Biology. 2025 Sep;100(3):161–87.
43. Kaun KR, Azanchi R, Maung Z, Hirsh J, Heberlein U. A Drosophila model for alcohol reward. Nat Neurosci. 2011 May;14(5):612–9.
44. Gibbons M, Versace E, Crump A, Baran B, Chittka L. Motivational trade-offs and modulation of nociception in bumblebees. Proceedings of the National Academy of Sciences. 2022 Aug 2;119(31):e2205821119.
45. Huemer M. Lexical Priority and the Problem of Risk. Pacific Philosophical Quarterly. 2010;91(3):332–51.
46. Fredrickson BL, Kahneman D. Duration neglect in retrospective evaluations of affective episodes. Journal of Personality and Social Psychology. 1993;65(1):45–55.
47. Redelmeier DA, Kahneman D. Patients’ memories of painful medical treatments: real-time and retrospective evaluations of two minimally invasive procedures. Pain. 1996 Jul 1;66(1):3–8.
48. Kahneman D, Fredrickson BL, Schreiber CA, Redelmeier DA. When More Pain Is Preferred to Less: Adding a Better End. Psychol Sci. 1993 Nov 1;4(6):401–5.
49. Redelmeier DA, Katz J, Kahneman D. Memories of colonoscopy: a randomized trial. Pain. 2003 Jul 1;104(1):187–94.
50. Auriemma CL, O’Donnell H, Jones J, Barbati Z, Akpek E, Klaiman T, et al. Patient perspectives on states worse than death: A qualitative study with implications for patient-centered outcomes and values elicitation. Palliat Med. 2022 Feb 1;36(2):348–57.
51. Patrick DL, Starks HE, Cain KC, Uhlmann RF, Pearlman RA. Measuring preferences for health states worse than death. Med Decis Making. 1994;14(1):9–18.
52. Wade JB, Hart RP. Attention and the stages of pain processing. Pain Med. 2002 Mar;3(1):30–8.
53. Alonso WJ, Schuck-Paim C. Pain-Track: a time-series approach for the description and analysis of the burden of pain. BMC Res Notes. 2021 Jun 5;14(1):229.
54. Schuck-Paim C, Alonso WJ, Hamilton C. Short agony or long ache: comparing sources of suffering that differ in duration and intensity [Internet]. 2024 [cited 2026 Jan 20]. Available from: https://welfarefootprint.org/2024/02/20/shortagony-or-longache/
55. Gómez-Emilsson A, Percy C. The Heavy-Tailed Valence Hypothesis: The human capacity for vast variation in pleasure/pain and how to test it [Internet]. PsyArXiv; 2022 [cited 2026 Jan 20]. Available from: https://osf.io/krysx_v1
Thanks for your post, Rob. Meghan Barrett and I have a detailed reply to Eisemann et al. 1984 in the Quarterly Review of Biology. You can see it here:
https://www.journals.uchicago.edu/doi/abs/10.1086/737365
Short version, very little in that paper has stood the test of time and the particular passage you quote has many problems. I’d encourage you to reconsider including it!
EDIT: Had some more thoughts that Substack won’t let me paste into a comment, so I put them in a doc: https://docs.google.com/document/d/1vhbCcV-EGhmm4c70BLp_6uY1jzOVzHIz84L1ePdMbvQ/edit?tab=t.0
A few points on the (farmed) insect vs shrimp comparison:
1. My understanding is that 99%+ of farmed insects are larvae, not adults. There's less evidence for the sentience of larvae. See:
https://forum.effectivealtruism.org/posts/yPDXXxdeK9cgCfLwj/short-research-summary-can-insects-feel-pain-a-review-of-the,
https://forum.effectivealtruism.org/posts/E7xdBbxqPNLjhrnz6/if-adult-insects-matter-how-much-do-juveniles-matter
(There may be more recent evidence since these, though.)
2. It wouldn't surprise me to find out that even if we ignored impacts on the insect larvae and considered only the adults, there would be more marginally cost-effective farmed insect (or even lab insect) interventions than our most marginally cost-effective shrimp ones, because the numbers are so large. (I don't have a strong opinion, and so far it seems it could go either way.)
3. My impression is that SWP's Humane Slaughter Initiative is highly scalable (to possibly millions of dollars per year) and its cost-effectiveness in terms of the number of animals helped/$ is not too speculative. On the other hand, we don't (yet) have anything like that for farmed insects, and instead it's a mix of many interventions, where each only scales so much, it's difficult to generalize across targets even for the same kind of intervention, and each intervention tends to be more speculative in terms of cost-effectiveness. However, it's plausible this will change soon after further research/R&D, and we could, for example, just pay producers to adopt more humane insect farming and slaughter practices.